Wild fruit diversity and the origins of cultivated trees
Wild fruit diversity in Central Asia and the Caucasus gave early cultivators unusually rich populations from which to select, move and propagate desirable trees, but modern genetics shows that high diversity is evidence of evolutionary history rather than proof of a single place of domestication. A 1931 survey treated the region’s wild apples, almonds, grapes, cherries, quinces and other fruits as clues to crop origins; several of those clues have since gained genetic support, while others have been revised.
This explainer places that historical survey in its scientific context, then compares its observations with genomic, archaeological and crop-wild-relative research. The focus is on what the old diversity patterns genuinely anticipated-especially for apples and grapes-and on why domestication is now understood as a long process involving selection, movement, hybridization and repeated gene flow rather than a simple one-location event.
Why the 1931 survey mattered
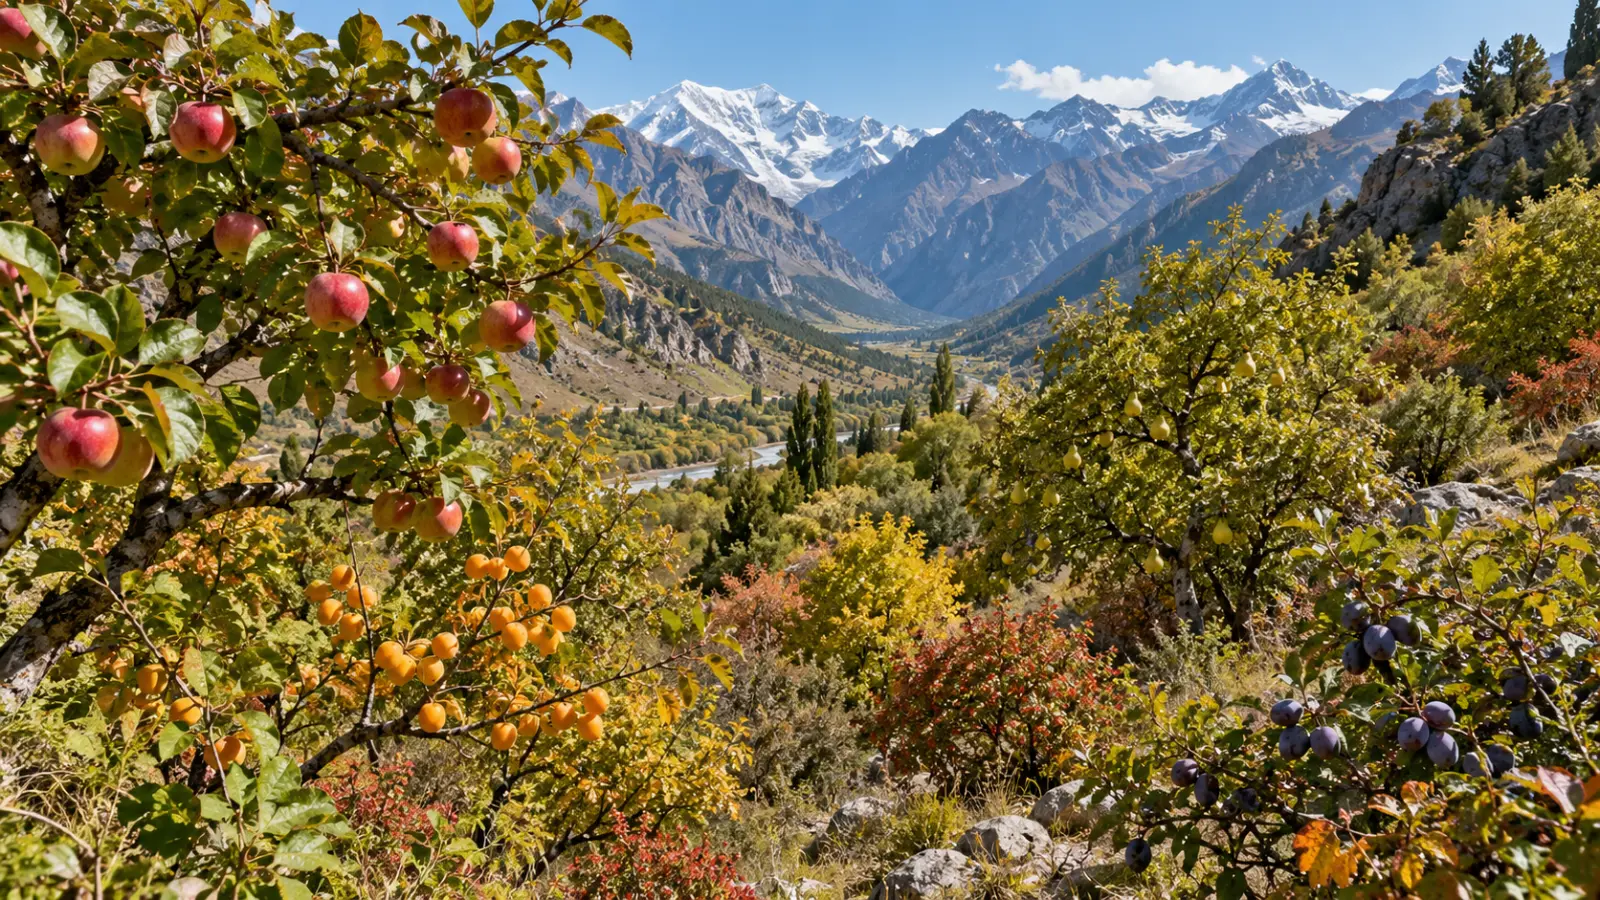
In 1931, N. I. Vavilov published an account of wild relatives of fruit trees in Turkestan and the Caucasus after years of plant-collecting work and comparison of crop variation across Eurasia. His central observation was geographic: some landscapes contained dense mixtures of wild and cultivated-looking forms, and variation often became narrower with distance from those concentrations. In the Caucasus he reported at least 80 wild species of fruits and nuts occurring together. He also described striking variation among indigenous grapes in Transcaucasia and highly variable wild almonds and apples in Turkestan.
For a geneticist working before DNA sequencing, those patterns were important evidence. N. I. Vavilov used morphology, geography, ecology and the presence of related wild forms to infer where crop diversity had accumulated and where domestication might have begun. Transitional forms between wild and cultivated plants, unusually large fruits in some wild populations, and the coexistence of many related taxa suggested long contact among natural populations, farmers and trade routes.
The 1931 paper therefore did more than catalogue species. It proposed a way to read landscapes as historical records. Modern research still uses geographic diversity, wild relatives and population structure, but it can now test the relationships with genome-wide markers, ancient plant remains and explicit demographic models. That has preserved the value of the observation while changing how confidently a diversity hotspot can be called an “origin.”
Diversity is a clue to domestication, not a one-to-one map
A region can be genetically or morphologically diverse for several reasons. It may contain a wild progenitor population; it may be a secondary zone where domesticated plants met wild relatives and exchanged genes; it may lie on a long-distance trade route; or it may simply contain many habitats that preserve old lineages. These processes can overlap. A high-diversity region can therefore be central to crop evolution without being the only place where people first domesticated the crop.
That distinction is one of the clearest differences between early twentieth-century “centres of origin” and current research on domestication. A 2021 global analysis by Maxted and Vincent of 1,425 crop wild relative species linked to 167 crops found substantial geographic overlap between wild-relative hotspots and classic centres of crop origin and diversity, while also identifying major differences and important hotspots outside them. The result supports N. I. Vavilov’s insight that diversity geography matters while showing why the boundaries and meaning of any single centre must remain testable rather than fixed.
Three mechanisms are especially important when interpreting old observations of “transitional” fruit forms:
- Selection from standing variation: people repeatedly favored larger, sweeter, less bitter, easier-to-harvest or more reliably fruiting individuals already present in diverse wild populations.
- Movement and mixing: seeds, cuttings and grafting material travelled with people, allowing cultivated lineages to meet distant wild populations and exchange genes.
- Clonal propagation: once a valuable fruit tree appeared, grafting or cuttings could preserve a genotype that would not breed true from seed, changing the pace and pattern of domestication.
Apple provides the clearest modern support for the Central Asian connection
Among the fruit trees discussed in the 1931 survey, apple offers the strongest example of a historical diversity observation later clarified by genomics. Modern cultivated apple, Malus domestica, has a major ancestral contribution from Malus sieversii, a wild apple distributed across Central Asia, especially Kazakhstan. A 2017 resequencing study of 117 diverse accessions supported a model in which cultivated apples arose primarily from M. sieversii and then acquired substantial genetic material from other wild apples as they moved westward along Eurasian exchange routes.
That later gene flow matters. European crabapple, Malus sylvestris, contributed substantially to the modern cultivated apple genome. This means that the “origin” of apple cannot be reduced to a single founding event followed by simple diffusion. A Central Asian progenitor relationship is strongly supported, yet the crop continued to evolve as humans transported it across landscapes containing compatible wild relatives. The diversity that N. I. Vavilov saw in Central Asia captured an important beginning, but not the whole history.
The same genetic complexity helps explain why wild apple populations remain valuable. Traits for disease resistance, climatic adaptation and fruit quality can exist in wild germplasm even when they are uncommon in commercial cultivars. Domestication selected a useful subset of diversity; conservation and breeding now depend on keeping access to the broader pool.
Grapevine links the Caucasus to an older and more complicated story
N. I. Vavilov treated the rich grape variation of Transcaucasia as another major clue. Archaeology and genetics confirm that the South Caucasus and wider Western Asian region are central to the early history of grape cultivation. McGovern et al. (2017) reported chemical and archaeobotanical evidence from Neolithic sites in Georgia indicating grape wine production around 6000–5800 BC, demonstrating an early, sustained relationship between people and grapevine in the region.
Genomics, however, has made the picture more network-like. A 2021 study of 204 Vitis vinifera genomes supported a Western Asian domestication event followed by extensive introgression from European wild grape populations. A separate review of grape domestication literature emphasized that the exact geographic extent, timing and number of domestication episodes have been debated because later breeding, trade and repeated wild-to-crop gene flow blur simple boundaries.
So the Caucasus remains highly relevant, but “high local diversity” and “single birthplace” are not interchangeable claims. The historical observation is strongest when framed as evidence that the region preserved deep wild and cultivated diversity and participated in early viticulture, not as proof that every cultivated grape lineage descends from one narrowly defined locality.
Almond, quince and cherry show both continuity and revision
The broader fruit-tree pattern is similar. Some crops fit the old geographic emphasis quite well; others reveal multiple contributors or uncertain boundaries when examined genetically.
Crop | 1931-era geographic clue | Modern evidence | Current interpretation |
Apple | Highly variable wild apples in Turkestan | Major ancestry from Malus sieversii in Central Asia, with later introgression from other wild apples | Central Asian ancestry combined with continued diversification during westward movement |
Grapevine | Exceptional diversity in Transcaucasian grapes | Early viniculture in the South Caucasus and genomic support for Western Asian ancestry | Early cultivation combined with later movement and introgression |
Almond | Variable wild almonds across Central Asian landscapes | Distinct cultivated clusters and several wild relatives across the Caucasus, Middle East and Central Asia | Multiple regional gene pools contributed to almond diversification |
Quince | Caucasus included among rich fruit-tree regions | Core origin area associated with Transcaucasia and northern Iran | Cultivation spread outward while preserving strong diversity in the original region |
Sweet cherry | Wild and cultivated fruit diversity around the Caucasus | Genomic evidence of domestication-related differentiation and reduced diversity in cultivated sweet cherry | Wild populations preserve extensive diversity alongside cultivated lineages |
Almond is a good example of why caution is necessary. A 2025 population-genetic study of 209 wild and cultivated almond accessions identified four cultivated genetic clusters and distinct gene pools among several wild relatives distributed across the Middle East and Central Asia. The authors found evidence consistent with complex relationships and gene flow, but they also concluded that more comprehensive sampling is needed to resolve almond domestication. That is more nuanced than assigning the crop to one centre based only on visible diversity.
Quince fits the Caucasian emphasis more closely. Modern reviews place the core area of origin in Transcaucasia and adjacent northern Iran, while also recognizing secondary diversity created as cultivation spread. Sweet cherry likewise has a long association with the zone between the Black and Caspian seas. A 2020 genome study found progressive losses of genetic variation from wild trees to landraces and modern varieties, consistent with domestication bottlenecks, while showing that wild populations still contain substantial diversity.
What N. I. Vavilov saw that modern genetics made testable
The most durable part of the 1931 argument is not any single boundary on a map. It is the relationship between wild diversity and crop history. N. I. Vavilov recognized that domesticated plants are embedded in broader species complexes and that geography can reveal where unusually rich variation has persisted. Modern genomics has turned those observations into testable hypotheses about ancestry, bottlenecks, introgression and selection.
Wild diversity was not a museum around domesticated crops; it was part of the evolutionary material from which many fruit crops were repeatedly selected, mixed and reshaped.
The word “repeatedly” is important. Tree crops are long-lived, often outcrossing, and frequently propagated vegetatively. Their domestication histories can span millennia and involve several layers: initial management of wild stands, selection of superior trees, clonal preservation, regional breeding, hybridization with wild relatives and movement across trade networks. Those layers make fruit-tree domestication especially likely to preserve signatures from multiple populations.
This is why modern studies often distinguish a progenitor population, a domestication zone, a centre of diversity and a later diversification region. They can overlap, but they are not synonyms. N. I. Vavilov’s field observations were strongest at identifying diversity-rich landscapes; DNA and archaeology are needed to determine what role each landscape played in a crop’s history.
What modern science changed
Several assumptions that were reasonable in 1931 now require tighter wording. First, visible similarity does not prove direct ancestry. Large-fruited wild trees can reflect natural variation, introgression from cultivation or independent evolution. Second, decreasing variation away from a hotspot can indicate dispersal, but trade, founder effects and later hybridization can produce similar gradients. Third, the taxonomic categories available to early researchers were based mainly on morphology, whereas genomic data can reveal hidden relationships or show that apparently similar forms have different histories.
Modern crop-domestication research therefore combines independent lines of evidence. Genome sequences estimate relatedness and past gene flow. Archaeobotanical remains provide dated evidence that people were using or managing particular plants. Historical linguistics, trade routes and written records can suggest movement, but they cannot substitute for biological evidence. Field collections remain essential because no genome study can recover diversity that has already disappeared from wild populations.
Seen this way, the 1931 survey is best treated as a historically important hypothesis-generating document. It correctly drew attention to Central Asia and the Caucasus as exceptional reservoirs of fruit-tree diversity. It should not be read as a final map of domestication events, because the modern evidence differs from crop to crop and often supports prolonged, reticulate histories rather than a single origin point.
Why the wild populations still matter
The scientific value of these regions is not only historical. Crop wild relatives can carry disease resistance, stress tolerance and other alleles that breeding populations may lack. As commercial orchards become genetically narrower and climates shift, those wild gene pools can provide options for breeding that were not needed-or not recognized-when older cultivars were selected.
Conservation is therefore part of the domestication story. Wild apple forests, grapevine populations, almond relatives and other fruit-tree communities are living archives of evolutionary variation. Protecting them in situ preserves ecological interactions and ongoing adaptation; maintaining well-documented ex situ collections provides material that breeders and researchers can compare and use. The two approaches are complementary.
The enduring lesson from the Turkestan and Caucasus survey is not that all fruit trees came from one vast centre. It is that unusually rich wild diversity can reveal where crop evolution has deep roots and where useful genetic variation still survives. Modern genetics has narrowed some hypotheses, complicated others and replaced a static map of origins with a dynamic picture of selection, movement and gene flow.
Frequently asked questions
Did N. I. Vavilov prove that cultivated fruit trees originated in the Caucasus and Turkestan?
No. The 1931 survey used geographic and morphological diversity to propose where important fruit-tree variation and possible progenitors were concentrated. Modern genetics supports major links for some crops, especially apple, but domestication often involved movement and gene flow. The historical paper is best read as a set of influential hypotheses, not a final map of origins.
Why is Malus sieversii important to the history of the cultivated apple?
Malus sieversii is a Central Asian wild apple that genomic studies identify as the major ancestral source of the cultivated apple. As apples moved westward, they also exchanged genes with other wild species, especially the European crabapple. Modern apple ancestry therefore combines a strong Central Asian origin with later introgression across Eurasia.
Does high wild diversity mean a crop was domesticated exactly where that diversity occurs?
Not necessarily. High diversity can mark a progenitor population, a long-term refuge, a secondary contact zone or a region where cultivated and wild plants repeatedly interbred. Trade and local adaptation can also create diversity after initial domestication. Researchers therefore combine genetics, archaeology and historical geography before assigning a domestication role to a region.
What did the Caucasus contribute to grapevine history?
The South Caucasus preserves deep grape diversity and contains some of the earliest archaeological evidence for viniculture, including Neolithic wine residues from Georgia. Genomic research also places major grape ancestry in Western Asia. Later movement and introgression from European wild grapes, however, mean that modern cultivars record a broader history than one isolated founding population.
Why do wild fruit relatives still matter to plant breeding today?
Wild relatives retain genetic variants that may be rare or absent in commercial orchards, including traits related to disease resistance and adaptation to heat, drought or other stresses. Conserving wild populations and germplasm collections gives breeders a wider genetic toolkit. Their value is practical as well as historical: they are resources for future crop improvement.
Sources
- N. I. Vavilov. Wild progenitors of the fruit trees of Turkistan and the Caucasus and the problem of the origin of fruit trees. Report and Proceedings of the 9th International Horticultural Congress, 1930. 1931:271–286. Record 19311600466.
- Duan N, Bai Y, Sun H, et al. Genome re-sequencing reveals the history of apple and supports a two-stage model for fruit enlargement. Nature Communications. 2017;8:249.
- Cornille A, Giraud T, Smulders MJM, Roldán-Ruiz I, Gladieux P. The domestication and evolutionary ecology of apples. Trends in Genetics. 2014;30(2):57–65.
- McGovern P, Jalabadze M, Batiuk S, et al. Early Neolithic wine of Georgia in the South Caucasus. Proceedings of the National Academy of Sciences. 2017;114(48):E10309–E10318.
- Magris G, Jurman I, Fornasiero A, et al. The genomes of 204 Vitis vinifera accessions reveal the origin of European wine grapes. Nature Communications. 2021;12:7240.
- Grassi F, De Lorenzis G. Back to the Origins: Background and Perspectives of Grapevine Domestication. International Journal of Molecular Sciences. 2021;22(9):4518.
- Abdollahi H. A review on history, domestication and germplasm collections of quince (Cydonia oblonga Mill.) in the world. Genetic Resources and Crop Evolution. 2019;66(5):1041–1058.
- Decroocq S, Cornille A, Dlalah N, et al. Insights Into the Almond Domestication History. Evolutionary Applications. 2025;18(9):e70150.
- Pinosio S, Marroni F, Zuccolo A, et al. A draft genome of sweet cherry (Prunus avium L.) reveals genome-wide and local effects of domestication. The Plant Journal. 2020;103:1420–1432.
- Maxted N, Vincent H. Review of congruence between global crop wild relative hotspots and centres of crop origin/diversity. Genetic Resources and Crop Evolution. 2021;68:1283–1297.
Lucas Merritt — author
Lucas writes animal science and zoology explainers. His editorial focus includes animal ecology, terrestrial and aquatic invertebrates, molluscs, invasive species, animal behaviour, species distributions and interactions between animals, agriculture and natura...
Related
Koshihikari rice: marker-assisted heading-date gene transfer
How vermicompost affects growth and flowering in Liatris spicata
Sugar components of coconut sugar in Indonesia: study digest
Can Alsike Clover Be Bred for Bulgaria’s Lowland Pastures?
How Tunisian Date Palm Seeds Differ in Chemistry and Bioactivity
Coffee, Cocoa and Tea: Cultivation, Management and Production